New version of the site! The interface has just been modernized — tell us what you think by email or rate it : ★★★★★ ★★★★★ ★ ★ ★ ★ ★ …
Marine Planktonic Copepods
Euchaeta marina  Prestandrea, 1833   (F,M1)
Taxonomy
Order Calanoida
Superfamily Clausocalanoidea
Family Euchaetidae

Synonymy

Cyclops marinus Prestandrea, 1833;
Euchaeta prestandreae Philippi, 1843; Claus, 1863 (p.183, 185, figs.F,M); Thompson, 1888 d (p.140); no Brady, 1883 (p.60); no ? King & Hida, 1955 (p.11);
E. communis Dana, 1849; Dahl, 1894 c (p.12, Rem.);
Euchäta marina : Giesbrecht, 1892 (p.262, 772, figs.F,M);
E. atlantica Lubbock, 1856;
E. sutherlandii Lubbock, 1856;
no E. marina : A. Scott, 1909 (p.67); Mori, 1937 (1964) (p.44, figs.F,M); Dakin & Colefax, 1940 (p.99, figs.F,M); Krishnaswamy, 1953 (p.117); ? King & Hida, 1955 (p.11); Yamazi, 1958 (p.148, Rem.); Grice, 1962 (p.199, fig.F); ? Ahlstrom & Thrailkill, 1963 (p.57, Table 5, abundance); Anraku & Azeta, 1965 (p.13, Table 2, fish predator); Tanaka & Omori, 1968 (p.220); ? Morris, 1970 (p.2300); Itoh, 1970 (p.4, Tab.1); Gueredrat, 1971 (p.300, fig.2, 10, Table 1, 2); ? Subbaraju & Krishnamurphy, 1972 (p.25, 26 ); Timonin, 1976 (p.79); Greenwood, 1977 (p.57, figs.F, Rem.); Chen Q-c, 1980 (p.795); Zheng Zhong & al., 1984 (1989) (p.237, figs.F,M); ? Williams D. & al., 1988 (p.580); ? Yoo, 1991 (tab.1); Arinardi, 1991 (p.295); He & al., 1992 (p.250); ? Shih & Young, 1995 (p.70); ? Wang & Zuo, 2004 (p.1, Table 2, dominance, origin); Takenaka & al., 2012 (p.1669, fig.2, 3, Table 1, bioluminescence assay); ? Noda & al., 1998 (p.55, Table 3, occurrence);

References

Giesbrecht & Schmeil, 1898 (p.38, Rem. F,M); I.C. Thompson, 1903 a (p.18); Thompson & Scott, 1903 (part., p.234, 244); Wolfenden, 1911 (p.299); ? Sewell, 1912 (? part., p.353, 360); ? Pesta, 1912 a (p.45); ? Sewell, 1914 a (p.215); Pesta, 1913 (p.32); 1920 (p.512); Sars, 1925 (p.104); Farran, 1929 (p.208, 237); Rose, 1929 (p.24); ? Sewell, 1929 (p.148); Sciacchitano, 1930 (p.15, figs.F,M); Pesta, 1943 (p.17, figs.M); Lysholm & al., 1945 (p.21); Sewell, 1947 (p.113, figs.F, Rem.); Brodsky, 1950 (1967) (p.198, figs.F,M); Marques, 1953 (p.99); 1958 (p.210); Heinrich, 1961 b (p.93); Vervoort, 1957 (p.76, Rem.); Chiba & al., 1957 (p.308); 1957 a (p.11); Fish, 1962 (p.13); Gaudy, 1962 (p.93, 99, Rem.: p.106, Pl.IV, Tableau 5: development: juv.); 1963 (p.23); Paiva, 1963 (p.41); Vervoort, 1963 b (part. p.158, Rem.); M. Bernard, 1964 (p.52, figs.N); Crisafi, 1965 b (p.263, figs.F,M, juv.); ? Saraswathy, 1966 (1967) (p.77); Owre & Foyo, 1967 (p.54, figs.F,M, Rem.); Mazza, 1967 (p.145, 161, F,M, juv.); 1968 (fiche CIESMM n°1); Ramirez, 1969 (p.63, figs.F,M); Shih & al., 1971 (p.39); Razouls, 1972 (p.94, Annexe: p.48, figs.F,M); Björnberg, 1972 (p.26, Rem.N, figs.); Kos, 1972 (Vol. I, figs.F, M, Rem.); Tanaka, 1973 (part., p.134, figs.F, Rem.); Marques, 1973 (p.238); 1974 (p.15); Bradford, 1974 (p.159, figs.F,M, fig.7, Rem.); Park, 1975 c (p.5, figs.F,M); ? Marques, 1976 (p.990); ? Tranter, 1977 (p.596); Björnberg & al., 1981 (p.633, 635, figs.F,M); ? Marques, 1982 (p.758); Sazhina, 1982 (p.1158, Rem., fig. N); 1985 (p.47, figs. N); Bradford & al., 1983 (p.18); Baessa de Aguiar, 1987 (p.41, figs.F, Rem.); Blades-Eckelbarger, 1991 (p.250, figs.M); Park, 1995 (p.15, Redescr.F,M, figs.F,M); Hure & Krsinic, 1998 (p.101); Mauchline, 1999 (n°182, p.8, figs.F,M); Bradford-Grieve & al., 1999 (p.880, 925, figs.F,M); Bragina, 1999 (p.195); Braga & al., 1999 (p.84, 86, 89, Rem.: Biol. mol., Table 1 , figs.6, 7, 8); G. Harding, 2004 (p.52, figs.F,M); Mulyadi, 2004 (p.71, figs.F,M, Rem.); Conway, 2006 (p.20, copepodides 1-6, Rem.); Avancini & al., 2006 (p.85, Pl. 54, figs.F,M, Rem.); Vives & Shmeleva, 2007 (p.649, figs.F,M, Rem.); Phukham, 2008 (p.119, figs.F)

Figures

Plate 1 issued from : Giesbrecht in M. Rose in Faune de France. 26- Copépodes pélagiques, Paul Lechevalier, Paris, 1933; [Fig.93, p.113].
Female and Male
Plate 2 issued from : J.M. Bradford in Pacific Science, 1974, 28 (2).[Fig.4, p.165; Fig.6, p.166].
Female: genital segment: a, dorsal view; b, left side; c, right side; d, ventral view.
Male: a, P5; b, serrate lamella of left P5 exopod segment 2.
Plate 3 issued from : T. Park in Bull. Scripps Inst. Oceanogr. Univ. California, San Diego, 1995, 29. [p.111, Fig.1].
Female: forehead (left side); b, urosome (left side); c, genital somite (left side); d, idem (dorsal); e, idem (right side); f, idem (ventral); g, caudal rami (dorsal); h, left caudal ramus (dorsal); i, idem (ventral); j, A1 (cut between segments 20 and 21); k, A2; l, Md; m, Mx1 (first inner lobe separated, posterior).
agf = anterior lobe of genital flange; ase = anterior seta; pgf = posterior lobe of genital flange; pse = posterior seta.

Nota: Laterally, forehead produced anteriorly into a large conical frontal eminence; Rostrum large pointing in an anteroventral direction, only slightly curved backward.
Distal margin of ptosome rounded; dorsally, posterolateral corners of prosome symmetrical and somewhat angular.
Genital somite in dorsal view strongly asymmetrical, with a large lobular outgrowth on right side and a small notch on left side. Laterally, right genital flange large, weakly bilobed; left genital flange smaller than right, clearly divided into a broad anterior and a narrow posterior lobe. Ventrally, posterior lobe of left genital flange extending mediad for only a short distance, leaving a relatively wide gap between it and medial edge of opposite genital flange. Within this gap and posterior to genital opening are seen conspicuous cuticular ridges.
4 distal marginal setae of caudal ramus about as long as urosome; appendicular caudal setae about 1.3 times length of body.
A1 extending beyond distal end of prosome by it last 3 segments.
In A2, outer margin of 2nd exopodal segment strongly bulging. Inner marginal seta of last exopodal segment well developed.
In Md, endopod reaching about middle of exopod.
In Mx1, 1st inner lobe with 1+9+1 (1 anterior + 9 marginal + 1posterior) setae; 1st endopodal segment with 1 seta, outer lobe with 5 setae.
Plate 4 issued from : T. Park in Bull. Scripps Inst. Oceanogr. Univ. California, San Diego, 1995, 29. [p.112, Fig.2].
Female: a, Mx2 (5th lobe and endopod separated, posterior); b, Mxp (coxa posterior, the rest anterior); c, P1 (anterior); d, P2 ( (anterior); e, P3 (anterior); f, P4 (anterior).
P1 = first leg; P2 = second leg; P3 = third leg; P4 = fourth leg.

Nota: In Mx2, 2 endopodal setae armed with long spinules in addition to very short spinules.
Basis of Mxp armed with long spinules in addition to rows of very small spinules along proximal half of medial margin.
Proximal, compound exopodal segment of P1, formed of first unseparated segments, with nearly straight outer margin and well-developed outer spine reaching about 2/3 way to base of following outer spine.
In P2 exopod, 2nd outer spine short of reaching base of following outer spine; 4th outer spine largest, a litthle short of reaching base of following outer spine; marginal lobe bearing 4th outer spine separated from segment by a deep and wide incision; marginal lobes carrying 2nd and 3rd outer spines separated from respective segments by a relatively deep cleft.
In P3 and P4, all outer spines of 3rd exopodal segment equally small.
Plate 5 issued from : T. Park in Bull. Scripps Inst. Oceanogr. Univ. California, San Diego, 1995, 29. [p.113, Fig.3].
Male: a, forehead (left side); b, last pedigerous and genital somites (left side); c, caudal rami (ventral); d, left caudal ramus (lateral); e, A2; f, Md; g, Mx1 (posterior); h, Mxp (coxa posterior, the rest anterior); i, first leg (anterior); j, second leg (anterior); k, 5th pair of legs (anterior); l, exopod of left 5th leg (anterior, tilted clockwise); m, idem medial, titled counterclockwise; n, distal end of serrated lamella (anterior).
dgp = digitiform process; htb = hairy tubercle; tsl = poorly sclerotized lobe.
Plate 6 issued from : F.C. Ramirez in Contr. Inst. Biol. mar., Buenos Aires, 1969, 98. [p.64, Lam. XII, figs.83, 90 ].
Male (from off Mar del Plata): 83, habitus (dorsal); 90, left P5 (detail of terminal exopodal segment)
Scale bars in mm: 1.5 (83).
Plate 7 issued from : F.C. Ramirez in Contr. Inst. Biol. mar., Buenos Aires, 1969, 98. [p.62, Lam. XI, fi.77].
Female (from off Mar del Plata): 77, urosome (lateral left side).
Scale bar in mm: 0.4.
Plate 8 issued from : R.B.S. Sewell in The John Murray Expedition, 1933-34, Scientific Reports, VIII (1), 1947. [p.114, Fig.25].
Female (from Arabian Sea): A, urosome with spermatophore (lateral right side); B, P1; C, P2 (in small form); D, P2 (in large form).
Nota: The proportional lengths of the various segments of the body (cephalon to caudal rami) in small example (3.0 mm) as 319:115:84:84:89:120:68:53:26:42 = 1000. In large example (3.683 mm) as 307:118:90:77:95:127:68:50:27:41 = 1000. There are also slight differences in the proportional lengths of the segments of A1; Differences can also be detected in the relative length of the 2nd spine on the external margin of the 3rd segment of the exopod of P2. In one specimen the joint between the 1st and 2nd segments of the exopod of P2 was incomplete, and the part of the combined segment that represented segment 1 was devoid of an inner seta.
The number of ova into egg-sacs was from 7 to 15 (mean 11), in every case the ovigerous female was also bearing one or more spermatophores (the maximum number observed on any single female was 11).
Plate 9 issued from : J. Mauchline in ICES Ident. Leafl. Plankton, 1999, N°182. [p.3, Fig.2: 2a-2b].
Female (Northeast Atlantic): a, genital double-somite (left side); b, same (dorsal).
Plate 10 issued from : J. Mauchline in ICES Ident. Leafl. Plankton, 1999, N°182. [p.4, Fig.3: 2c].
Male (Northeast Atlantic): 2c, terminal two segments, exopodal segments of left P5.
Plate 11 issued from : G. Harding in Key to the adullt pelagic calanoid copepods found over the continental shelf of the Canadian Atlantic coast. Bedford Inst. Oceanogr., Dartmouth, Nova Scotia, 2004. [p.52].
Female & Male.

Nota: Female with deep incision, in lateral view) between frontal organ and rostrum (arrowed). Two of the six apical setae on Mx2 bearing long spines in addition to short spinules (arrowed).
Plate 12 issued from : T. Park in Smiths. Contr. Zool., 1975, 196. [p.5, Fig.1].
Female (G. of Mexico): a, forehead (lateral); b, genital segment (ventral).

Male: c, forehead (lateral); d, exopod of left P5 (anterior).
Plate 13 issued from : H.B. Owre & M. Foyo in Fauna Caribaea, 1967, 1, Crustacea, 1: Copepoda. [p.55, Figs.332-335].
Female (from Florida Current): 332, Mx2.

Male: 333, right P5; 334, left P5; 335, terminal segments of left P5.
Plate 14 Issued from : W. Giesbrecht in Systematik und Faunistik der Pelagischen Copepoden des Golfes von Neapel und der angrenzenden Meeres-Abschnitte. – Fauna Flora Golf. Neapel, 1892, 19 , Atlas von 54 Tafeln. [Taf.37, Figs.37, 38]. As Euchäta marina.
Female: 37, urosome (lateral); 38, same (ventral).
Plate 15 Issued from : W. Giesbrecht in Systematik und Faunistik der Pelagischen Copepoden des Golfes von Neapel und der angrenzenden Meeres-Abschnitte. - Fauna Flora Golf. Neapel, 1892, 19 , Atlas von 54 Tafeln. [Taf.37, Fig.49]. As Euchäta marina.
Female: 49, forehead (lateral).
R = rostrum.
Plate 16 Issued from : W. Giesbrecht in Systematik und Faunistik der Pelagischen Copepoden des Golfes von Neapel und der angrenzenden Meeres-Abschnitte. - Fauna Flora Golf. Neapel, 1892, 19 , Atlas von 54 Tafeln. [Taf.37, Fig.30]. As Euchäta marina.
Female: 30, caudal rami and setae (ventral).
Nota: Se = outer seta; St = terminal seta.
Plate 17 Issued from : W. Giesbrecht in Systematik und Faunistik der Pelagischen Copepoden des Golfes von Neapel und der angrenzenden Meeres-Abschnitte. - Fauna Flora Golf. Neapel, 1892, 19 , Atlas von 54 Tafeln. [Taf.37, Fig.30]. As Euchäta marina.
Female: 30, caudal rami (ventral; magnified).
Plate 18 Issued from : W. Giesbrecht in Systematik und Faunistik der Pelagischen Copepoden des Golfes von Neapel und der angrenzenden Meeres-Abschnitte. - Fauna Flora Golf. Neapel, 1892, 19 , Atlas von 54 Tafeln. [Taf.16, Fig.30]. As Euchäta marina.
Female: 30, A1 (segments 1 to 18; ventral view).
S di = distal seta.
Plate 19 Issued from : W. Giesbrecht in Systematik und Faunistik der Pelagischen Copepoden des Golfes von Neapel und der angrenzenden Meeres-Abschnitte. - Fauna Flora Golf. Neapel, 1892, 19 , Atlas von 54 Tafeln. [Taf.16, Fig.30]. As Euchäta marina.
Female: 30, A1 (segments 17 to 24-25; ventral view).
S di = distal seta; S pr = proximal seta.
Plate 20 Issued from : W. Giesbrecht in Systematik und Faunistik der Pelagischen Copepoden des Golfes von Neapel und der angrenzenden Meeres-Abschnitte. - Fauna Flora Golf. Neapel, 1892, 19 , Atlas von 54 Tafeln. [Taf.16, Figs.1, 2]. As Euchäta marina.
Female: 1, A2 (posterior view); 2, A2 (anterior view).
Plate 21 Issued from : W. Giesbrecht in Systematik und Faunistik der Pelagischen Copepoden des Golfes von Neapel und der angrenzenden Meeres-Abschnitte. - Fauna Flora Golf. Neapel, 1892, 19 , Atlas von 54 Tafeln. [Taf.16, Fig.41]. As Euchäta marina.
Female: 41, Mx1 (anterior view).
B2 = basis; Li 2 = inner lobe 2.; Ri = endopod.
Plate 22 Issued from : W. Giesbrecht in Systematik und Faunistik der Pelagischen Copepoden des Golfes von Neapel und der angrenzenden Meeres-Abschnitte. - Fauna Flora Golf. Neapel, 1892, 19 , Atlas von 54 Tafeln. [Taf.16, Fig.28]. As Euchäta marina.
Female: 28, Mx2 (posterior view).
Plate 23 Issued from : W. Giesbrecht in Systematik und Faunistik der Pelagischen Copepoden des Golfes von Neapel und der angrenzenden Meeres-Abschnitte. - Fauna Flora Golf. Neapel, 1892, 19 , Atlas von 54 Tafeln. [Taf.16, Fig.8]. As Euchäta marina.
Female: 8, Mxp (B1 anterior view, rest posterior view).
Plate 24 Issued from : W. Giesbrecht in Systematik und Faunistik der Pelagischen Copepoden des Golfes von Neapel und der angrenzenden Meeres-Abschnitte. - Fauna Flora Golf. Neapel, 1892, 19 , Atlas von 54 Tafeln. [Taf.15, Fig.31]. As Euchäta marina.
Female: 31, exopod of P1 (posterior view).
Plate 25 Issued from : W. Giesbrecht in Systematik und Faunistik der Pelagischen Copepoden des Golfes von Neapel und der angrenzenden Meeres-Abschnitte. - Fauna Flora Golf. Neapel, 1892, 19 , Atlas von 54 Tafeln. [Taf.16, Fig.46]. As Euchäta marina.
Female: 46, exopodite 2 and 3 of P2 (posterior view)
Plate 26 Issued from : W. Giesbrecht in Systematik und Faunistik der Pelagischen Copepoden des Golfes von Neapel und der angrenzenden Meeres-Abschnitte. - Fauna Flora Golf. Neapel, 1892, 19 , Atlas von 54 Tafeln. [Taf.16, Fig.15]. As Euchäta marina.
Female: 15, exopodal outer margin of P3 (posterior view).
Se = outer seta.
Plate 27 Issued from : W. Giesbrecht in Systematik und Faunistik der Pelagischen Copepoden des Golfes von Neapel und der angrenzenden Meeres-Abschnitte. - Fauna Flora Golf. Neapel, 1892, 19 , Atlas von 54 Tafeln. [Taf.16, Fig.22]. As Euchäta marina.
Female: 22, exopodal outer margin of P4.
Plate 28 Issued from : W. Giesbrecht in Systematik und Faunistik der Pelagischen Copepoden des Golfes von Neapel und der angrenzenden Meeres-Abschnitte. - Fauna Flora Golf. Neapel, 1892, 19 , Atlas von 54 Tafeln. [Taf.16, Fig.29]. As Euchäta marina.
Male: 29, A1 (ventral view).
Ae = aestherasc; S di = distal seta; Spr = proximal seta.
Plate 29 Issued from : W. Giesbrecht in Systematik und Faunistik der Pelagischen Copepoden des Golfes von Neapel und der angrenzenden Meeres-Abschnitte. - Fauna Flora Golf. Neapel, 1892, 19 , Atlas von 54 Tafeln. [Taf.16, Figs.16, 17]. As Euchäta marina.
Male: 16, right P5 (posterior view); 17, left P5.
Plate 30 Issued from : W. Giesbrecht in Systematik und Faunistik der Pelagischen Copepoden des Golfes von Neapel und der angrenzenden Meeres-Abschnitte. - Fauna Flora Golf. Neapel, 1892, 19 , Atlas von 54 Tafeln. [Taf.16, Fig.25]. As Euchäta marina.
Male: 25, exopodite 2 and 3 of left P5.
Plate 31 Issued from : W. Giesbrecht in Systematik und Faunistik der Pelagischen Copepoden des Golfes von Neapel und der angrenzenden Meeres-Abschnitte. - Fauna Flora Golf. Neapel, 1892, 19 , Atlas von 54 Tafeln. [Taf.15, Fig.33]. As Euchäta marina.
Male: 33, exopod of P1 (posterior view).
Plate 32 Issued from : W. Giesbrecht in Systematik und Faunistik der Pelagischen Copepoden des Golfes von Neapel und der angrenzenden Meeres-Abschnitte. - Fauna Flora Golf. Neapel, 1892, 19 , Atlas von 54 Tafeln. [Taf.16, Fig.23]. As Euchäta marina.
Male: 23, outer margin of exopodite 2 and 3 of P2.
Plate 33 issued from : P.E. Lapernat & C. Razouls in Vie Milieu, 2002, 52 (1). [p.28, Pl. VI, fig.10].
Masticatory edge of Md gnathobase female (from off Malta, Mediterranean Sea).

Nota: Itoh's index: 858.9 (number of teeth: 7).
Plate 34 issued from : P.E. Lapernat & C. Razouls in Vie Milieu, 2002, 52 (1). [p.21, Pl. II, fig.6].
Masticatory edge of Md gnathobase female (from off Malta, Mediterranean Sea).
Nota: The Itho's index vale for the the mandibular gnathobase = 858.9.
Plate 35 issued from : R. Gaudy in Rev. Trav. St. Mar. End., Bull. 27 (42). [p.128, Tableau 5].
Identification of copepodids stages Euchaeta marina.
A: Stage; B: number of swimming legs; C: number of thoracic segments; D: number of abdominal segments; E, Size.
Plate 36 issued from : N. Phukham in Species diversity of calanoid copepods in Thai waters, Andaman Sea (Master of Science, Univ. Bangkok). 2008. [p.212, Fig.86].
Female (from W Malay Peninsula):a, habitus (dorsal); b, forehead (lateral); c-d, genital segment (lateral and dorsal, respectively); e, P2.

Body length after drawing: F = 3.375 mm.
Plate 37 issued from : O. Tanaka in I O B C Handbook, 1973, IV. [p.134, Fig.4]. With doubt. Not taken into account by Park (1995, p.15)).
Female (from Indian Ocean); A, forehead (lateral); B-D, genital segments for different specimens.

Nota: There is some doubt concerning a good identification of this species because possible confusion with the allied forms E. marinella and E. rimana.
Plate 38 issued from : O. Tanaka in I O B C Handbook, 1973, IV. [p.148, Fig.9: 1]. With doubt. Not taken into account by Park (1995, p.15).
Female: 1, genital segment (dorsal).

Nota: Genital segment asymmetrical, produced on the right side about the middle.
Plate 39 issued from : Mulyadi in Published by Res. Center Biol., Indonesia Inst. Sci. Bogor, 2004. [p.71, Fig.40].
Female (from Indonesian Seas): a, habitus (dorsal); b, forehead (lateral); c, posterior part of last thoracic segment and genital complex (lateral right side); d, P2.

Male: e, habitus (dorsal); f, forehead (lateral); g, posterior part of last thoracic segment and genital somite (lateral left side); h, P5; i, exopod of left P5.
Plate 40 Issued from : T. Park in Smithsonian Contr. Zool., 1975, 196. [p.5, Fig.1].
Female (from G. of Mexico & Caribbean Sea): a, forehead (lateral); b, genital segment (ventral).

Male: c, forehead; d, exopod of left P5 (anterior).

Nota: In the Gulf of Mexico and western Caribbean Sea, this species is the most common euchaetid in the epipelagic zone; although its batymetrical distribution extends occasionally down to a depth of about 500 m, its main concentration usually appears between depths of 25 and 100 m.
Plate 41 Issued from : T. Park in Antarctic Res. Ser., 1978, 27 (4). [p.206, Fig.65].
Female (from 26°36'S, 36°41'W & 36°42'S, 53°09'W): A, forehead (lateral; B-E, distal end of metasome and genital segment (dorsal, left side, right side, and ventral, respectively); F, outer lobe of Mx1; G, P1 (anterior); H, P2 (anterior).
Plate 42 Issued from : T. Park in Antarctic Res. Ser., 1978, 27 (4). [p.206, Fig.65].
Male (from 26°36'S, 36°41'W & 36°42'S, 53°09'W): A, forehead (lateral); B, last metasomal and genital segment (lateral); C, P5 (anterior); D, middle part of exopod of left P5 (anterior); E, middle part of exopod of left P5 (medial).

Nota : Proportional lengths of prosome and urosome about 70 : 30 :
Forehead similar to that of female, but frontal eminence pointing downward and rostrum curved backward.
Last metasomal segment prolonged posteriorly on each side into lappet covering about ½ of genital segment; Laterally, posterodorsal margin bearing toothlike process.
P5 biramous left and right. Right endopod slightly longer 1st exopodal segment. Left endopod rudimentary. Distal exopodal segment of right leg tapering into spiniform process longer than rest of leg. 2nd segment of left exopod with elongated hollow serrated lamella, slender digitiform process, and small conical tubercle. 3rd segment of left exopod a little shorter than rest of leg, consisting of hollow proximal portion and long tapering distal part ; tuft of spinules and digitiform process present at junction of these two parts.
Plate 43 issued from : J.M. Bradford in Pacific Science, 1974, 28 (2). [p.166, Fig.5, a].
Female: c, genital field and right border of genital segment.

Nota:
Genital field in ventral view with genital pads not meeting in midline, gap between them about 1/2 width of right pad.
Plate 44 Euchaeta marina Female:
1 - See Key to marina species Group.
2 - Laterally, genital somite less than 1.5 times as long as deep (Fig.1-b).
3 - In P2 exopod, 2nd outer spine of 3rd segment longer than outer spine of 2nd segment (Fig.2-d).
4 - Ventrally, genital field with wide gap between genital flanges (Fig.1-f).
Plate 45 issued from : J.M. Bradford in Pacific Science, 1974, 28 (2). [p.164, Fig.2].
Female (from 28°35'N, 73°33W): Mx1.
Plate 46 issued from : J.M. Bradford in Pacific Science, 1974, 28 (2). [p.164, Fig.3].
Comparison between exopods of P1 and P2 female of Euchaeta marina (a, b), Euchaeta rimana (c, d) and Euchaeta marinella (e, f).

Nota: Exopod of P1: Bb ± 2/3 BC, Cc ± 4/3 BC. Exopod of P2: Aa ≤ AB, Bb ± 1/2 BC, Cc ≤ CD.
In E. rimana P1 exopod: Bb ±2/3 BC, Cc ≥ BC.
In E. marinella exopod of P1: Bb ≥ 1/2 BC, Cc ≥BC; exopod of P2: Aa ± 3/4 AB, Bb ≤ 1/2 BC, Cc ≤ 1/2 CD.
Plate 47 issued from : J.M. Bradford in Pacific Science, 1974, 28 (2). [p.167, Table 2]
Female and Male: comparison between Euchaeta marina and allied forms.
Plate 48 Issued from : M.S. Kos in Field guide for plankton. Zool Institute USSR Acad., Vol. I, 1972. After Brodsky, 1962.
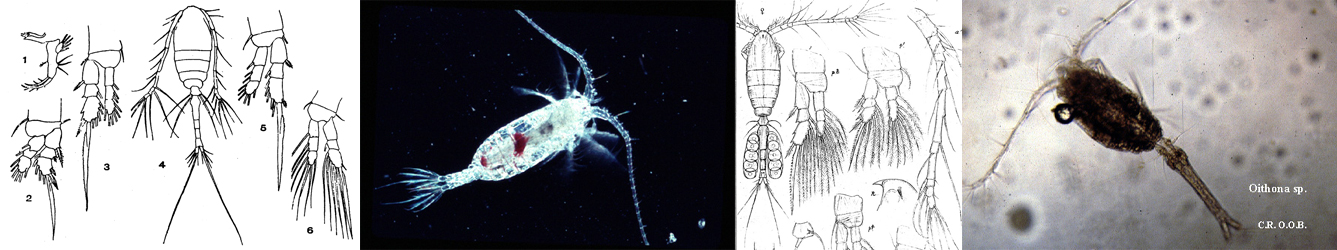
Female: 1, habitus (dorsal) with eggss; 2, habitus (lateral); 3, forehead (lateral); 4, urosome (lateral); 5, genital segment; 6, P2; 7, P1.
Male: 8, habitus (lateral); 9, distal end of exopod (serrated lamelle nA) of P5.
Plate 49 Issued from : G. Belmonte in The Eur. Zool. J., 2018, 85 (1). [p.274, Fig.1].
Euchaeta marina (Prestandrea, 1833).
a, first nauplius; b, metanauplius; c, Mxp; d, extremity of A1- d1 female, d2 male; c, 5th pair of thoracic legs, male; f, caudal ramui- f1 female, f2 male; g, adult male (lateral view); h , adult female (lateral view). (Redrawn from different sources: a from Sazhina 1985; b from Bjornberg, 1972; c-g from Giesbrecht 1892; h: from Claus, 1863.

Complementary References

Cleve, 1904 a (? part., p.190); Pearson, 1906 (p.16, Rem.); ? Cazrl, 1907 (p.15); Rose, 1925 (p.152); Massuti Alzamora, 1942 (p.90); Wilson, 1942 a (part., p.185); Oliveira, 1945 (p.191); Wilson, 1950 (part. p.214); Deevey, 1960 (p.5, Table II, annual abundance); ? Fagetti, 1962 (p.21); ? Ganapati & Shanthakumari, 1962 (p.8, 15); Cervigon, 1962 (p.181, tables: abundance distribution); Grice & Hart, 1962 (p.287, table 3); V.N. Greze, 1963 a (tabl.2); Gaudy, 1963 (p.23, Rem.); Björnberg, 1963 (p.37, Rem.); Unterüberbacher, 1964 (p.23); ? De Decker & Mombeck, 1964 (p.12); Shmeleva, 1965 b (p.1350, lengths-volume-weight relation); ? Mullin, 1966 (p.546, Table I, III, diet); Dawson, 1966 (p.176); Pavlova, 1966 (p.43); Neto & Paiva, 1966 (p.23, Table III); Chakroun, 1966 (p.67, Table); ? Furuhashi, 1966 a (p.295, vertical distribution in Kuroshio region, Table 9); Mazza, 1966 (p.70); 1967 (p.367); Ehrhardt, 1967 (p.738, figs.12, 51-53, geographic distribution, Rem.); ? Grice & Hulsemann, 1967 (p.16); ? Fleminger, 1967 a (tabl.1); ? Itoh, 1970 (tab.1); Vinogradov, 1968 (1970) (p.78, 80, 278); Evans, 1968 (p.13); Dowidar & El-Maghraby, 1970 (p.268); Park, 1970 (p.476); Deevey, 1971 (p.224); Carli, 1971 (p.373, tab.2); Salah, 1971 (p.319); ? Timonin, 1971 (p.281, trophic group); Roe, 1972 (p.277, tabl.1, tabl.2); 1972 b (p.526); Brodsky, 1972 (P.256); Apostolopoulou, 1972 (p.327, 347); Binet & al., 1972 (p.71); Bainbridge, 1972 (p.61, Appendix Table I: vertical distribution vs day/night, Table II:%, Table IV: thermal stability vs upwelling); Ibanez & Seguin, 1972 (p.81, annual cycle, multivarite analysis); ? Heinrich, 1973 (p.95); ? Björnberg, 1973 (p.329, 386); ? Patel, 1975 (p.659); Gaudy, 1975 (p.109, fig.1, Table I, 4, respiration); Ikeda, 1976 (p.51, respiration rate); ? Frontier, 1977 a (p.14); Deevey & Brooks, 1977 (p.256, tab.2, Station "S"); ? Timonin & Voronina, 1977 (p.290, fig.7); Carter, 1977 (1978) (p.35); Arashkevich, 1978 (p.118, Table: diets); ? Stephen & Iyer, 1979 (p.228, tab.1, 3, 4, figs.3, 4); Dessier, 1979 (p.201, 205); Vaissière & Séguin, 1980 (p.23, tab.2); Svetlichnyi, 1980 (p.28, Table 1 as Fuchaeta marina, passive submersion); Sreekumaran Nair & al., 1981 (p.493, fig.2cont.); Madhupratap & al., 1981 (p.262, Table 2: abundance vs. thermocline); Madhupratap & al., 1981 (p.266, fig.2j: abundance vs. geographic transect); Kovalev & Shmeleva, 1982 (p.83); Kovalev & Shmeleva, 1982 (p.83); Gaudy & Boucher, 1983 (p.37, Table 1, 2, 3, 5, figs.1, 2, Rem.: metabolism); Minkina, 1983 (p.38, speed swimming); ? Guangshan & Honglin, 1984 (p.118, tab.);Tremblay & Anderson, 1984 (p.5); De Decker, 1984 (p.316, 349: chart); Cummings, 1984 (p.163, Table 2); Scotto di Carlo & al., 1984 (p.1042); Kinzer & Schulz, 1985 (tab.4); Regner, 1985 (p.11, Rem.: p.31); Longhurst, 1985 (tab.2); Brenning, 1985 a (p.23, Table 2); Sazhina, 1985 a (p.491, tab.3); Petipa & Borichenko, 1985 (tab.1,2); Moraitou-Apostolopoulou, 1985 (p.303, occurrence/abundance in E Mediterranean Sea); Jansa, 1985 (p.108, Tabl.III, V); Sarkar & al., 1986 (p.178); Shuert & Hopkins, 1987 (p.49); Shuert & Hopkins, 1987 (p.30, feeding: diet composition); Renon, 1987 (tab.2); Gorsky & al., 1988 (p.133, Table I, C-N composition); Lozano Soldevilla & al., 1988 (p.58); Hernandez-Trujillo, 1989 a (tab.1); Cervantes-Duarte & Hernandez-Trujillo, 1989 (tab.3); Herman, 1989 (p.247); Mitra & al., 1990 (fig.3); Suarez & al., 1990 (tab.2); Othman & al., 1990 (p.565, Rem.); Gajbhiye & al., 1991 (p.189); Lindo, 1991 (tab.3); Suarez & Gasca, 1991 (tab.2); Hernandez-Trujillo, 1991 (1993) (tab.I); Samba Diouf, 1991 (p.104); Huntley & Lopez, 1992 (p.201, Table B1, growth rate, temperature-dependent production); Suarez, 1992 (App.1); Seguin & al., 1993 (p.23); Hays & al., 1994 (tab.1); Kouwenberg, 1994 (tab.1); Roff & al., 1995 (p.165, Table 1, 3, 5, nauplii development times, nauplii copepodites growth rates, naupllii vs. bacteriophagy/picoplankton, naupliar production); Webber & Roff, 1995 a (p.481, table 1, 2, 3, 6, 7, 8, biomass, production); Palomares Garcia & Vera, 1995 (tab.1); ? Kotani & al., 1996 (tab.2); Webber & al., 1996 (tab.1); Suarez-Morales & Gasca, 1997 (p.1525); Sharaf & Al-Ghais, 1997 (tab.1); ? Go & al., 1997 (tab.1); ? Hwang & al., 1998 (tab.II); Gilabert & Moreno, 1998 (tab.1,2); Mauchline, 1998 (tab.63, 30, 42, 47, 64, 65); Alvarez-Cadena & al., 1998 (tab.1,2,3,4); Suarez-Morales, 1998 (p.345, Table 1); Suarez-Morales & Gasca, 1998 a (p.109); Hopcroft & al., 1998 (tab.2); Lapernat, 1999 (p.17, 55); Siokou-Frangou, 1999 (p.476); Hernandez-Trujillo, 1999 (p.284, tab.1); Lavaniegos & Gonzalez-Navarro, 1999 (p.239, Appx.1); El-Serehy, 1999 (p.172, Table 1, occurrence); Lopes & al., 1999 (p.215, tab.1); Neumann-Leitao & al., 1999 (p.153, tab.2); Lapernat, 2000 (tabl.3, 4); Suarez-Morales & al., 2000 (p.751); Fernandez-Alamo & al., 2000 (p.1139, Appendix); Plounevez & Champalbert, 2000 (p.175, Table III, IV, V, abundance vs fish); ? Escribano & Hidalgo, 2000 (p.283, tab.2); Suarez-Morales & Gasca, 2000 (1247, tab.1); Suarez-Morales & al., 2000 (p.751, tab.1); Seridji & Hafferssas, 2000 (tab.1); Lopez-Salgado & al., 2000 (tab.1); Hidalgo & Escribano, 2001 (p.159, tab.2); Hidalgo & Escribano, 2001 (p.158, fig.5); Lapernat & Razouls, 2001 (tab.1); Hernandez-Trujillo & Suarez-Morales, 2002 (p.748, tab.1); Beaugrand & al., 2002 (p.179, figs.5, 6); Pusch & al., 2004 (251, tab.3); CPR, 2004 (p.54, fig.155); Kazmi, 2004 (p.229); Dias & Bonecker, 2005 (p.100 + poster); Alvarez-Silva & al., 2005 (p.39); Ashjian & al., 2005 (p.1380: tab.2); Berasategui & al., 2005 (p.313, fig.2); ; Manning & Bucklin, 2005 (p.233, Table 1); Dias Araujo, 2006 (p.49, Rem., chart); Durbin & Casas, 2006 (p.2537, Table 2b); Lopez-Ibarra & Palomares-Garcia, 2006 (p.63, Tabl. 1, seasonal abundance vs El-Niño, Rem.: p.70, 72); Khelifi-Touhami & al., 2007 (p.327, Table 1); Jitlang & al., 2008 (p.65, Table 1); Fernandes, 2008 (p.465, Tabl.2); McKinnon & al., 2008 (p.844: Tab.I, p.848: Tab. IV); Neumann-Leitao & al., 2008 (p.799: Tab.II, fig.6); Morales-Ramirez & Suarez-Morales, 2008 (p.513); Muelbert & al., 2008 (p.1662, Table 1); Gaard & al., 2008 (p.59, Table 1, N Mid-Atlantic Ridge); ? Pagano, 2009 (p.116); Miyashita & al., 2009 (p.815, Tabl.II); C.E. Morales & al., 2010 (p.158, Table 1); Hafferssas & Seridji, 2010 (p.353, Table 3); Schnack-Schiel & al., 2010 (p.2064, Table 2: E Atlantic subtropical/tropical); Hernandez-Trujillo & al., 2010 (p.913, Table 2); Hidalgo & al., 2010 (p.2089, Table 2); Sun & al., 2010 (p.1006, Table 2); Dias & al., 2010 (p.230, Table 1); Mazzocchi & Di Capua, 2010 (p.425); Medellin-Mora & Navas S., 2010 (p.265, Tab. 2); Fazeli & al., 2010 (p.153, Table 1); ? Maiphae & Sa-ardrit, 2011 (p.641, Table 2); Andersen N.G. & al., 2011 (p.71, Fig.3: abundance); Selifonova, 2011 a (p.77, Table 1, alien species in Black Sea); Shiganova & al., 2012 (p.61, Table 4); Uysal & Shmeleva, 2012 (p.909, Table I); Mulyadi & Rumengan, 2012 (p.202, Rem.: p.204); Miloslavic & al., 2012 (p.165, Table 2, transect distribution); Naz & al., 2012 (p.61, Table 4, relative abundance); Hidalgo & al., 2012 (p.134, Table 2) ; Belmonte & al., 2013 (p.222, Table 2, abundance vs stations); Teuber & al., 2013 (p.28, Table 1, respiration rates); Teuber & al., 2013 (p.1, Table 1, 2, 3, fig.5, abundance vs oxygen minimum zone, respiration rates, enzyme activity); in CalCOFI regional list (MDO, Nov. 2013; M. Ohman, comm. pers. [see in Remarks]); Melo Jùnior & al., 2013 (p.363, Table 2, egg production); Lidvanov & al., 2013 (p.290, Table 2, % composition); Bonecker & a., 2014 (p.445, Table II: frequency, horizontal & vertical distributions); Lopez-Ibarra & al., 2014 (p.453, Table 2, biogeographical affinity); Mazzocchi & al., 2014 (p.64, Table 5, abundance); Dias & al., 2015 (p.483, Table 2, abundance, biomass, production); Bode & al., 2015 (p.268, Table 1, chemical components, trophic level, geographic zone); Zakaria & al., 2016 (p.1, Table 1); Benedetti & al., 2016 (p.159, Table I, fig.1, functional characters); Marques-Rojas & Zoppi de Roa, 2017 (p.495, Table 1); Jerez-Guerrero & al., 2017 (p.1046, Table 1: temporal occurrence); El Arraj & al., 2017 (p.272, table 2, spatial distribution); Benedetti & al., 2018 (p.1, Fig.2: ecological functional group); Belmonte, 2018 (p.273, Table I: Italian zones); Abo-Taleb & Gharib, 2018 (p.139, Table 5, occurrence %); Chaouadi & Hafferssas, 2018 (p.913, Table II: occurrence); Bode & al., 2018 (p.840, Table 1, fig.5 as spp., respiration & ingestion rates); Acha & al., 2020 (p.1, Table 3: occurrence % vs ecoregions, Table 5: indicator ecoregions).
Distribution

Additional Maps & Charts

Map 5 issued from : J.M. Bradford in Pacific Science, 1974, 28 (2). [Fig.7, p.167).
Distribution of Euchaeta marina, E. rimanaand E. marinella based on specimens seen by the author.
Map 6 issued from : T.S.K. Björnberg in Bol. Inst. Oceanogr., Sao Paulo, 1963, XIII (1). [p.38, Fig.20].
Probability of occurrence of Euchaeta marina in different environments.
T: Tropical waters (above 36.00 p.1000 salinity and above 20°C temperature); SST: Surface subtropical waters (salinity around 36 p.1000 and temperature 18°C or less); DST: Deeper shelf waters (salinity between 34 and 36, temperature under 20°C p.1000); SS: Surface shelf waters (same salinity and temperature above 20°C);
C: coastal waters with low salinity and variable temperature.

In each column no shading means no probability of finding the species in the samples from this environment; horizontal shading indicates the probability of finding the sepecies in percentages less than one in samples from this environment; cross shading indicates the probability of finding it in percentages higher than one and black shading represents the probability of finding it in the largest percentages of the total number of copepods.

Nota: The histogram shows this species as a copepod which prefers warm, very saline waters, therefore thermophile. As it did not occur in coastal waters it is preferentially a shelf oceanic species in Brazilian waters. It occurred in small quantities or not at all in the samples from deeper layers: therefore a surface copepod.
Map 7 issued from : H.B. Owre & M. Foyo in Fauna Caribaea, 1967, 1, Crustacea, 1: Copepoda. [p.54, Table 20].
Vertical distribution of Euchaeta marina.
Samples collected at the 40-mile Station in the Florida Current (18 may 1958).
A: 10.37-13.27 h; B: 22.59-01.18 h.
Map 8 issued from : A.A. Shmeleva in Bull. Inst. Oceanogr., Monaco, 1965, 65 (n°1351). [Table 6: 20 ]. Euchaeta marina (from South Adriatic).
Dimensions, volume and Weight wet. Means for 50-60 specimens. Volume and weight calculated by geometrical method. Assumed that the specific gravity of the Copepod body is equal to 1, then the volume will correspond to the weight.
Map 9 issued from : U. Brenning in Wiss. Z. Wilhelm-Pieck-Univ. Rostock - 33. Jahrgang 1981. Mat.-nat. wiss. Reihe, 6. [p.2, Fig.1].
T-S Diagram for Euchaeta marina, E. acuta, E. hebes (= Paraeuchaeta hebes), E. paraconcinna from Cap Blanc (Mauritania).
SO: Southern Surface Water (S °/oo: 34,50; T°C: 29,0); ND: Northern Water of the Surface Layer (S °/oo: 37,5; T°C: 21,0); SD: Southern Deep Water of the surface layer (S °/oo: 35,33; T°C: 13,4). See commentary in Temora stylifera and Brenning (1985 a, p.6).
Map 10 Issued from : M.K. Webber & J.C. Roff in Mar. Biol., 1995, 123. [p.484, Table 1].
Length-weight regression of Euchaeta marina in oceanic waters of Discovery Bay (Jamaica) in 60- and 200 m vertical hauls, using 200- and 64-µm mesh aperture of plankton nets, from June 1989 to July 1991 (monthly samples).
Map 11 Issued from : M.K. Webber & J.C. Roff in Mar. Biol., 1995, 123. [p.485, Table 2].
Mean biomass (µg) of copepodite stages for Euchaeta marina from Discovery Bay (Jamaica), with standard deviation and n number of individuals measured.
Map 12 Issued from : M.K. Webber & J.C. Roff in Mar. Biol., 1995, 123. [p.485, Table 3].
Stage weight increments (In mmax mmin-1) for Euchaeta marina from Discovery Bay (Jamaica) calculated from mean biomass of each stage.
Map 13 Issued from : M.K. Webber & J.C. Roff in Mar. Biol., 1995, 123. [p.487, Table 4].
Stage duration (days) for copepodite stages of Euchaeta marina from Discovery Bay (Jamaica), n: number of observations.
Map 14 Issued from : M.K. Webber & J.C. Roff in Mar. Biol., 1995, 123. [p.487, Table 5].
Mean number of eggs per female for Euchaeta marina, and corrected egg development time in days. n: number of observations.
Map 15 Issued from : M.K. Webber & J.C. Roff in Mar. Biol., 1995, 123. [p.488, Table 6].
Estimates of generation times (in days) from egg to first egg clutch for Euchaeta marina from Discovery Bay (Jamaica), based on minimum and maximum development time of individual life history stages. Centering indicates Max and Min values identical.
Map 16 Issued from : M.K. Webber & J.C. Roff in Mar. Biol., 1995, 123. [p.488, Table 7].
Growth coefficient (g) and daily specific growth rate (G) for Euchaeta marina from Discovery Bay (Jamaica).
Map 17 Issued from : M.K. Webber & J.C. Roff in Mar. Biol., 1995, 123. [p.487, Table 8].
Euchaeta marina: Minimum female weight (MFW), mass of eggs (M of E) and mass of female and eggs (MF + E) all in µg AFDW. Growth coefficient (g) and daily specific growth rate (G) for eggs.
AFDW = ash-gree dry weight.
Map 18 Issued from : M.K. Webber & J.C. Roff in Mar. Biol., 1995, 123. [p.483].
Equations used for the estimation of Euchaeta marina production as for other copepods in the Discovery Bay (Jamaica).
Map 19 Issued from : M.K. Webber & J.C. Roff in Mar. Biol., 1995, 123. [p.483].
Equations used for estimation of egg production in Euchaeta marina as for other copepods from Discovery Bay (Jamaica)
Map 20 Issued from : J.C. Roff, J.T. Turner, M.K. Webber & R.R. Hopcroft in Aquat. microb. Ecol., 1995, 9. [p.170, Table 5].
Summary observations on naupliar bacterivory on FLB (fluorescently labelled bacteria) a partir Escherichia coli (±0.7 µm3 cell volume) in Discovery Bay (Jamaica).
Fluorescence levels: 0 = no materal for observation; - = no fluorescence observed; + = low fluorescence due to few FLB observe; * = highly fluorescence due to many FLB.

The authors show of the 11 species examined (Centropages velificatus, Acartia lilljeborgi, Paracalanus aculeatus, Temora stylifera, Undinula vulgarius, Euchaeta marina, Clausocalanus spp., Onaea sppp., Corycaeus spp.), 7 showed clear evidence of feeding on FLB (see table 5), with 92% of their nauplii ingesting FLB, clearly visible in the guts of many nauplii, and usually comprisised a discrete feeding (foregut) or 'fecal' (hindgut) bolus of cells. After only 30 min, fecal pellets were being produced already filled with FLB. Presence of FLB in guts cannot be interpreted as incidental feeding or 'drinking', because 4 species failed to ingest them (Centropages velificatus, Euchaeta marina, Clausocalanus sp., Corycaeus sp.). The very earliest stages may not ingest bacteria or other particles because they may have yolk reserves (for example Temora turbinata N1 nauplii did not ingest FLB, but later stage nauplii did).
Map 21 Issued from : M. Bode, R. Koppelmann, L. Teuber, W. Hagen & H. Auel inGlobal Biogeochemical Cycles, 2018, 32. [p.844, Table 1).
Cf. explanations of these measures in Calanoides natalis from the same authors.
Compare with Paraeuchaeta gracilis, P. aequatorialis.

Localisations

South Africa (W, S, E), Atlant. (tropical, sub-tropical), Namibia, Atlant. (central equatorial), Angola, Baia Farta, Congo, G. of Guinea, off Lagos, Ivorian shelf, Dakar, off NW Cape Verde Is., Morocco- Mauritania, Great Meteor Seamount, Canary Is., Azores, Gibraltar, Argentina, Uruguay (continental shelf), Brazil (S, off Macaé, off Rio de Janeiro, Campos Basin, Cabo Frio, off Vitoria-Cabo de Sao Tomé, off Natal), off Amazon, Barbada Is., Caribbean Sea, Caribbean Colombia, Bahia de Mochima (Venezuela), Cariaco Basin, Yucatan, Jamaica (Discovery Bay), Yucatan (Ascension Bay), E Costa Rica, G. of Mexico, Louisiana (off Grand Isle), Florida, Sargasso Sea, off Bermuda: Station "S" (32°10'N, 64°30'W), Delaware Bay (outside), G. of Maine, off Woods Hole, Georges Bank, G. of St. Lawrence, off S Iceland, W Ireland, off SW Ireland, Faroe Is., North Sea, Medit. (Alboran Sea, Habibas Is., Sidi Fredj coast, Algiers, Gulf of Annaba, Castellon, Baleares, Banyuls, G. of Lions, Marseille, Villefranche-s-Mer, Ligurian Sea, Tyrrhenian Sea, Messina, Gulf of Taranto, Tripoli, Malta, Adriatic Sea, Ionian Sea, Aegean Sea, Black Sea, Lebanon Basin, W Egyptian coast, Alexandria), Hurghada, N Red Sea, Gulf of Oman, ? Arabian Sea, ? Arabian Gulf, UAE coast, Karashi coast, ? Natal, ? Madagascar (Nosy Bé), ? Kavaratti & Agatti Is., ? off Cochin, ? equatorial Indian Ocean, ? India (Saurashtra coast, Porto Novo, Bombay, Lawson's bay, Hooghly estuary), E India, ? Bay of Bengal, Andaman Sea, W Malay Peninsula (Andaman Sea), Bali Sea, ? Ambon Bay, Flores Sea, Australia (North West Cape, ? G. of Carpentaria in Markina, 1972b, ? Great Barrier, Gulf of Tonkin in Brodsky, 1972 (p.256); ? Pacif. (E & W equatorial) (in Guangshan & Honglin, 1984), [ ? Korea (in Park & Choi, 1997), Yellow Sea in Sun & al., 2010; ? E China Sea (Kuchinoerabu Is.), ? Japan, ? Okinawa ], California, W Baja California (in Ahlstrom & Thrailkill, 1963); , Bahia Magdalena, W (in Lopez-Ibarra & Palomares-Garcia, 2006; Hernandez-Trujillo & al., 2010), G. of California (in Jimenez-Perez & Lara-Lara, 1988), W Mexico (in Suarez-Morales & al., 2000), G. of Tehuantepec, off W Guatemala, Costa Rica (Dome), Clipperton Is., Bahia Cupica (Colombia) ? Peru, Chile (N-S, Santiago, Concepcion)

Quotations

N: 513 ? (any confusion with E. rimana in the Indian Ocean and probably in the East tropical Pacific)

Dimensions (mm)

(3) F: 3,64-3,4; M: 3,2-2,88; (14) F: 3,3-2,73; M: 3,1-2,85; (19) F: 2,84-3,44; M: 2,88-3,4; (47) F: 3,9-2,25; M: 3,2-3,05; (73) F: 3,53; M: 3,59; (199) F: 3,57-3,19; M: 3,19-3,04; (207) F: 3,56-3,48; M: 3,52-3,3; (237) F: 3,3; M: 2,8-3,0; (244) F: 3,2-2,8; (340) M: 3,5; (432) F: 3,9-3,5; (449) F: 3,9-2,25; M: 3,2-3 ; ?(530) F: 3,8; M: 3,5; (785) F: 3,36-2,59; M: 3,18-2,56; (864) F: 2,86-3,38; (920) F: 3,33; (1111) F: 2,93-3,65; M: 2,6-3,81; (1122) F: 3,2; M: 2,45; (1230) F: 3,0-3,7; M: 3,1-3,7; {F: 2,25-3,90; M: 2,56-3,81}

The mean female size is 3.268 mm (n = 29; SD = 0.4513), and the mean male size is 3.117 mm (n = 24; SD = 0.3393). The size ratio (male : female) is 0.967 (n = 9; SD = 0.478), or ± 97 %. In samples, the sex ratio (female : male) is 1.214, but likely 1.

Prosome length: (19) F: 2,08-2,48; M: 2,12-2,36.

Remarks

Oceanic, epi-mesopelagic, 300 m (off Malta). Sargasso Sea: 0-1500 m (Deevey & Brooks, 1977, station "S").
For Park (1995, p.14) this species belongs to ‘’marina’’ Group, characterized by : Two endopodal setae of Mx2 armed with long spinules in addition to short spinules. Basis of Mxp with long spinules in addition to short spinules along proximal half of medial margin. Exopod of male left P5 with 3 poorly sclerotized lobes : 1/- next to digitiform process of 2nd segment ; 2/- on hairy tubercle ; 3/- next to tufts of stiff hairs on 3rd segment. In exopod of male left P5, digitiform process spiniform and serrated lamella long, extending beyond tufts of stiff hairs.
Bradford (1974) puts doubt on the cosmopolitan distribution of this species by the establishment of two new species in Indonesia and the Pacific: E. rimana and E. marinella. The geographic distribution of E. marina appears to be essentially Atlantic and Mediterranean (Park, 1995), and, without doubt in the Indian Ocean. This in spite of the fact that Madhupratap & Haridas (1986) do not cite the species. Possible distribution in the East-Pacific, although the species is not counted by Hernandez-Trujillo & Esqueda-Escarcega, 2002 (in Appendix: p.62). Cited as abundant by Lopez-Ibarra & Palomares-Garcia (2006, Table 1); Hernandez-Trujillo & Suarez-Morales (2002) along the west coast of South California. The locality records in the NW and SE Pacific also call for a serious confirmation. This species is not mentioned in the Fauna of Japan by Chihara & Murano, 1997.
Occurrence confirmed in the Chinese Seas by W. Zhang (pers comm., 2010). Palomares-Garcia & al., 2018 (p.178, Table 1: not occurrence of this species in the La Paz Bay from 1987 to 2011, where a doubtful identification and possible confusion with Euchaeta rimana) in the NE tropical Pacific, as Lopez Ibarra (2008).
See in Remarks to Euchaeta rimana.
After Park (1975 c, p.5) this species is the most common euchaetid in the epipelagic zone in the Gulf of Mexico and western Caribbean Sea.
According to Owre & Foyo (1967, p.54) the majority of specimens was collected in the upper 200 m in the Florida Current. The depth range can be between 0-1316 m, but over 96 % of the specimens were obtained from the upper 100 m.
After Shiganova & al. (2012, p.99) this species new in the Black Sea (as other species) arise from a rise of the water surface layer temperature and/or increasing of shipping activity during the last decades.
For Itoh (1970 a, fig.2, from co-ordonates) the Itoh's index value of the mandibular gnathobase = 740 (a doubt subsists concerning the species), and for Gaudy & Boucher (1983, p.43, Table 5) = 750.

After Shuert & Hopkins (1987, p.55) in the eastern Gulf of Mexico, the diet composition study of this specie, based on fore-and mid-gut contents, indicated that adult female ingest small crustaceans, primarily copepods. Adult males appeared not to feed. Histological examination revealed thin, thread-like guts which contained no food. Feeding appendages, for example the mandible and maxillipeds, were noticeably reduced in sized compared to those of females and younger male stages.

After Ehrhardt (1967, p.888, 894) the species is found in the southwest Tyrrhenian Sea in water salinity between 37.08-38.35 p.1000 (mainly between 37.78- 37.91) and for the Oxygen between 4.43-6.00 cm3/l (mainly between 4.70-5.45).
Timonin (1971, p.282) considers the trophic interrelations in the equatorial and tropical Indian Ocean, and divides the plankters into 6 trophic groups from the litterature and the results of studies of mouth-parts structure and intestine content. This species is a seizing and masticating carnivorous.
After Park (1995, p.16) this species was found widely in the Atlantic between 39°N and 33°S.
After Benedetti & al. (2018, p.1, Fig.2) this species belonging to the functional group 1 corresponding to large sac-spawning carnivorous.
Last update : 28/10/2022

Contributor Remarks

 to add your remark